In this post I'll do a few very explicit computations for motivic cell structures of smooth projective toric varieties coming from the Białynicki-Birula decomposition, namely P1,P1×P1,P2 and Hirzebruch surfaces. It is a bit lengthy but maybe helpful to anyone who wants to do some explicit calculations with BB-decompositions. I hope you're accustomed to toric varieties, but I won't do anything fancy. You can safely skip the motivic part of this post.
I wrote about motivic cell structures and the Białynicki-Birula decomposition before. Here I'll explain how to compute a motivic cell structure out of the BB-decomposition explicitly and how to get an explicit BB-decomposition for any smooth complete toric variety. Then I'll do the examples.
Explicit Motivic Cell Structure
As described in the last post about Białynicki-Birula's Annals paper from 1972/73, for a Gm-action on a smooth complete variety X over a (possibly non-closed) field k (of arbitrary characteristics), there is the plus-decomposition, giving us for each fixed point a∈XGm a subscheme Xa+⊂X which is isomorphic to an affine space Xa+≃Ana. The number na is the dimension of the positive weight part (with respect to the induced Gm-action) of the (co)tangent space of X at a.
There is another paper of Białynicki-Birula, published in 1976 in the Bulletin de l'académie polonaise des sciences, Série des sciences math., where it is proved that the BB-decomposition of smooth projective varieties is filtrable, which means that one can choose an order on the fixed points XGm={a0,…,am} and a partition of m into d blocks (where d is the dimension of X) such that for Xi the union of cells of each block, the Xi are closed subschemes of X that form a finite decreasing sequence !X=Xd⊃Xd−1⊃⋯⊃X0⊃X−1=∅. Here every ⊃ is a proper inclusion. The proof uses Sumihiro's equivariant completion, which provides an equivariant closed immersion into a projective space with linear torus action, so there one can filter the projective space by the weights of this action and that provides the closed immersions. If one wants to compute something, one can of course figure out a good order of the fixed points by hand, without looking at equivariant embeddings at all. At the moment, I don't know any algorithm other than brute force to do that.
Now we build a motivic cell structure out of this. This is slightly unusual, as the attaching maps arise "the other way around" than one would expect. If it confuses you, the examples below might provide illumination. The open subscheme X∖Xi→X∖Xi−1 has complement isomorphic to a disjoint union of some Xai+. Look at the closed immersion of smooth schemes ι:Xai+→X∖Xi−1 and its normal bundle Nι. By the homotopy purity theorem of Morel and Voevodsky we have !Nι/(Nι∖Xai+)=:Th(Nι)≃(X∖Xi−1)/((X∖Xi−1)∖ι(Xai+)!=(X∖Xi−1)/(X∖Xi)≃S2ni,ni. If we want to handle more cells at once, we just define Th(Ni) by X∖Xi→X∖Xi−1→Th(Ni) to be a homotopy cofiber sequence. One more homotopy cofiber construction gives us Th(Ni)→Σ(X∖Xi), an attaching map of Th(Ni)∼⋁S2nα,nα into Σ(X∖Xi) that gives us, as next homotopy cofiber, the space Σ(X∖Xi−1). So this produces inductively a stable motivic cell structure on X, since for A→B→C a cofiber sequence with two stably cellular spaces, a theorem of Dugger and Isaksen shows that the third space is also stably cellular.
That toric varieties have a motivic cell structure (without referring to the BB-decomposition) is already contained in the paper of Dugger and Isaksen Motivic Cell Structures.
Motives
From a homotopy cofiber sequence X→Y→Z→⋯ we get a distinguished triangle in the category of motives DM− of the reduced motives h~(X)→h~(Y)→h~(Z)→[1]⋯. Like with reduced and unreduces cohomology theories, h~(Y)⊕Z=h(Y), so we can compute motives of varieties from homotopy cofiber sequences.
Concrete Gm-actions with isolated fixed points
It is long known for toric varieties, that any torus cocharacter in general position (in the cocharacter lattice) has the same fixed points as the torus. To describe explicit cell decompositions, one needs to know which cocharacter is "in general position" and which cocharacter has a larger fixed point set. A cocharacter α fixes an orbit Oτ if α is inside the linear subspace generated by τ. The full torus has as fixed points those Oτ with τ of maximal dimension. To pick a good cocharacter, one just has to avoid the hyperplanes spanned by the codimension 1 cones in the fan.
The Projective Line
The fan of the projective line consists of the cone {0} and the cones generated by 1 and −1 respectively. The affine variety corresponding to the 1-cone is A01:=P1∖{∞}⊂P1 and the affine variety corresponding to the −1-cone is A∞1:=P1∖{0}⊂P1. Their intersection is the affine variety corresponding to the cone {0}, which is the torus Gm=P1∖{0,∞}.
The torus Gm acts on itself via the group multiplication, and it acts on {0} and {∞} trivially, i.e. these are the fixed points of the action. If you prefer homogeneous coordinates, λ∈Gm(k) acts on [x:y]∈P1(k) as λ.[x:y]=[λx:y], so we have λ.[0:1]=[0:1] and λ.[1:0]=[λ:0]=[1:0].
The Kähler differentials are ΩP1/k,01≃ΩA01/k,01=⟨dX⟩k and ΩP1/k,∞1≃ΩA∞1/k,01=⟨dX−1⟩k. The induced Gm(k)-action is λ.dX=λdX and λ.dX−1=λ−1dX−1, respectively. We see that the positive weight part at 0 is everything, while at ∞ it is nothing. Consequently, the orthogonal at 0 is nothing and at ∞ it is everything. Under m→m/m2 we get an isomorphic preimage of this orthogonal and take the ideal generated by it. This gives us ideals n0=(0) and n∞=(X−1). They correspond to the cells X0+=V(n0)=A01 and X∞+=V(n∞)={∞}.
This is already the BB-decomposition: P1=A1∪{∞}. The BB-filtration X=Xd⊃Xd−1⊃⋯⊃X0⊃X−1=∅. of X=P1 is (with d=1) just P1⊃{∞}. To get a motivic cell structure, we need attaching maps for the cell Th(Nι)≃X/X0=P1≃S2,1 to the set of 0-cells X0={∞}. The stable attaching map is the cofibration S2,1→Σ(P1∖{∞}), which one can see as the homotopy cofiber of P1→P1, i.e. the gluing of P1 along ∞ to a point ∞.
The homotopy cofiber sequence yields a distinguished triangle !h~(P1)→h~(S2,1)→h~(Σ(P1∖{∞}))→h~(P1)[1]→⋯ which we can identify as !h~(P1)→Z(1)[2]→0→⋯. Now we have a splitting h~(P1)=Z(1)[2].
We can also take a different Gm-action on P1, by taking any cocharacter (i.e. group homomorphism) Gm→Gm. These are all of the form λ↦λn for some n∈Z. If n>0, we get the same weight decomposition of (co)tangent spaces (Kähler differentials), hence the same BB-decomposition. If n=0, we get no decomposition because the fixed points are not isolated (they are everything). If n<0, we get the decomposition P1={0}∪A∞1, which one might also call the minus-decomposition w.r.t. the first action considered.
A product of two lines
Here we have a torus Gm×Gm acting and it becomes a slightly more interesting question which cocharacter Gm→Gm×Gm gives which BB-decomposition.
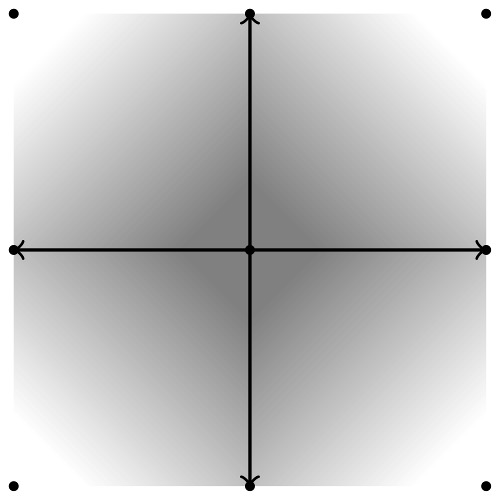
The fixed points of the torus are the orbit closures corresponding to the maximal cones, which are (0,0),(0,∞),(∞,∞),(∞,0).
Take the diagonal λ↦(λ,λ) corresponding to the weight (1,1) in the weight lattice. It doesn't hit any linear subspace generated by codimension one cones, so it has the same isolated fixed points, as the original torus. (In contrast, e.g. λ↦(λ,1) fixes a whole {0}×P1).
From analyzing the positive weight subspaces of the cotangent spaces of P1×P1 at these fixed points, we get (Ω(0,0)1)+=⟨dX,dY⟩k (Ω(0,∞)1)+=⟨dX⟩k (Ω(∞,∞)1)+=0 (Ω(∞,0)1)+=⟨dY⟩k and from this the ideals defining the cells n(0,0)=(0)≤k[X,Y] n(0,∞)=(Y−1)≤k[X,Y−1] n(∞,∞)=(X−1,Y−1)≤k[X−1,Y−1] n(∞,0)=(X−1)≤k[X−1,Y] so the cells are X(0,0)+=A01×A01 X(0,∞)+=A01×{∞} X(∞,∞)+={(∞,∞)} X(∞,0)+={∞}×A01
It is pretty obvious now how much influence the choice of a cocharacter has on the cell decomposition. There are only four different cell decompositions, corresponding to the four maximal-dimensional cones in the fan.
The BB-filtration is P1×P1⊃P1×{∞}∪{∞}×P1⊃{(∞,∞)}⊃∅. The motivic cell structure is built inductively, we start with the cellular space {(∞,∞)}≃A1×A1 and attach the cellular space Th(N1)≃S2,1∨S2,1 to it (to obtain P1×P1∖{(∞,∞)}) via the homotopy cofiber sequence !A1×A1→P1×P1∖{(∞,∞)}→Th(N1)→Σ(A1×A1). In the next step we attach to the stably cellular space P1×P1∖{(∞,∞)} the cellular space Th(N0)≃S4,2 to obtain P1×P1 via the homotopy cofiber sequence !P1×P1∖{(∞,∞)}→P1×P1→Th(N0)→Σ(P1×P1∖{(∞,∞)}).
This is also the motivic cell structure you would get as product cell structure from the previously considered cell structure for P1, and it is all parallel to classical topology, up to homotopy (though classically the gluing maps don't look that strange).
For the sake of completeness, let's compute the motive from this (i.e. let's look at the distinguished triangles): !0→h~(P1×P1∖{(∞,∞)}))→Z(1)[2]⊕Z(1)[2]→0→⋯ shows that h~(P1×P1∖{(∞,∞)}))=Z(1)[2]⊕Z(1)[2], as expected from the observation P1×P1∖{(∞,∞)})≃P1∨P1≃S2,1∨S2,1. The next homotopy cofiber sequence gives !Z(1)[2]⊕Z(1)[2]→h~(P1×P1)→Z(2)[4]→Z(1)[3]⊕Z(1)[3]→⋯ and we get h~(P1×P1)=Z(1)[2]⊕Z(1)[2]⊕Z(2)[4], since there are no non-trivial morphisms Z(2)[4]→Z(1)[3].
The Projective Plane
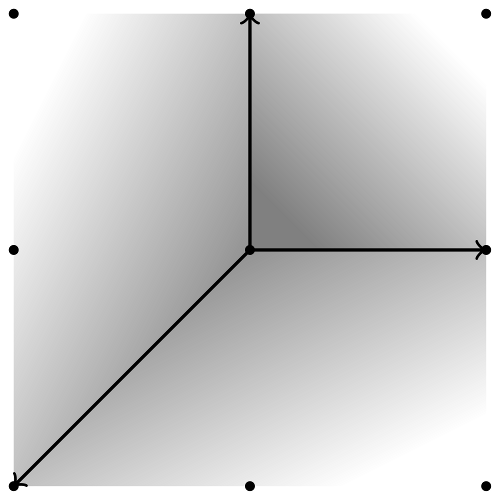
The fixed points of the torus Gm×Gm are [0:0:1], [1:0:0] and [0:1:0] (corresponding to the maximal dimensional cones 1,2,3 in the fan, in counter-clockwise order). Denote by Ui the affine toric variety corresponding to the maximal dimensional cone i.
The cotangent spaces at the fixed points are ΩP2,[0:0:1]=ΩU1,(0,0)=⟨dX,dY⟩k, ΩP2,[1:0:0]=ΩU2,(0,0)=⟨dX−1Y,dX−1⟩k, ΩP2,[0:1:0]=ΩU3,(0,0)=⟨dXY−1,dY−1⟩k.
The diagonal cocharacter λ↦(λ,λ) is no longer good, since (1,1) lies in the linear subspace generated by a cone of the fan -- it fixes the projective line {[x:y:0]∣[x:y]∈P1}.
We can choose the cocharacter λ↦(λ−1,λ), which acts with the same isolated fixed points as the whole torus on P2. For this one we get: (Ω[0:0:1]1)+=⟨dY⟩k, (Ω[1:0:0]1)+=⟨dX−1Y,dX−1⟩k, (Ω[0:1:0]1)+=0, so that we have cells X[0:0:1]+=V(X)={[0:y:1]∣y∈A1}⊂U1, X[1:0:0]+=V(0)=U2≃A2, X[0:1:0]+={[0:1:0]}. This decomposition is one of the common decompositions of P2 into A2 and a P1 at infinity, which is decomposed into A1 and ∞. The corresponding BB-filtration is just P2⊃P1⊃P0.
The homotopy cofiber sequences that give the motivic cell structure are !A2→P2∖P0→Th(N1)≃S2,1→ΣA2 !P2∖P0→P2→Th(N0)≃S4,2→Σ(P2∖P0). As before, we have h~(P2∖P0)=Z(1)[2] and h~(P2)=Z(1)[2]⊕Z(2)[4].
If we pick another cocharacter λ↦(λ−2,λ−1), this is still inside the cone 2, but it has a different scalar product with one of the rays, so the decomposition should be different. Indeed, from computations we find that the big cell now is part of U3 and in U2 we have only a 0-cell.
Hirzebruch surfaces
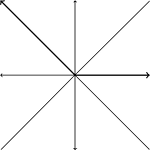
The fan for a Hirzebruch surface Fa=P(O(a)⊕O) looks similar to the fan of P1×P1=P(O⊕O):
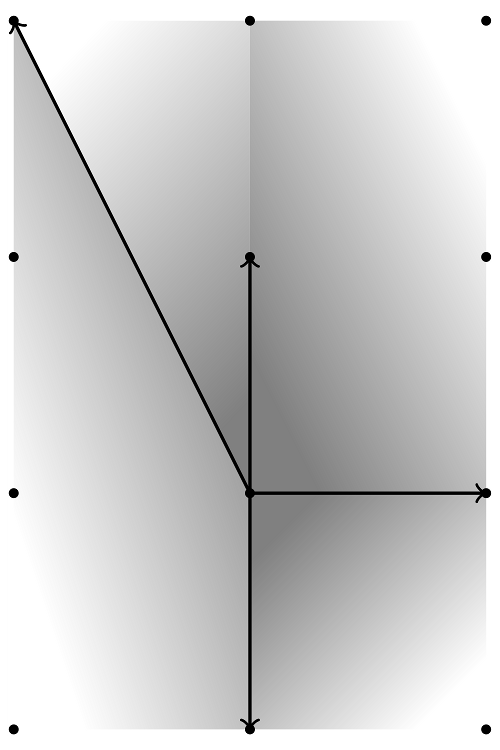
The image shows the fan of F2.
We pick the torus cocharacter of weight (1,1) again, since it works for all Hirzebruch surfaces.
The cone generated by (0,1) and (1,0) as well as the cone generated by (1,0) and (0,−1) are just as in the situation of F0=P1×P1, and the corresponding affine toric varieties glue together to a P1×A1, which is visible in the cell structure. The big cell is A2 corresponding to the cone with faces (0,1) and (1,0).
The cone generated by (−1,a) and (0,−1) corresponds to a fixed point which is a BB-cell itself and the cone generated by (0,1) and (−1,a) corresponds to a fixed point with attached BB-cell of dimension 1.
The BB-filtration is Fa=X2⊃X1⊃X0⊃∅ with X0 the fixed point which already is a cell and X1 everything except the big cell (big cell = unique open cell). The motivic cell structure is built from the homotopy cofiber sequences !A2→Fa∖X0→Th(N1)→ΣA2 !Fa∖X0→Fa→Th(N0)→Σ(Fa∖X0). The space Fa∖X0 is homotopy equivalent to the P1 at the base, but the gluing map Th(N0)→Σ(Fa∖X0) really depends on a.
The motive is just the same as the motive of P1×P1.
More complete nonsingular surfaces
It is a well-known fact (and not hard to prove) that all complete nonsingular toric surfaces (implicitly assuming normal) are either P2, a Hirzebruch surface Fa or a blow-up of one of these at torus fixed points, since one can describe such blow-ups with fans. One easily sees that blowing up a fixed point introduces an additional fixed point with "BB-cell" A1, therefore an additional S2,1 to the motivic cell structure (the additional P1). This introduces an additional Z(1)[2] to the motive.
 Konrad Völkel